Deer Behavior Affects Density Estimates With Camera Traps, but Is Outweighed by Spatial Variability
Abstract
Density is a key trait of populations and an essential parameter in ecological research, wildlife conservation and management. Several models have been developed to estimate population density based on camera trapping data, including the random encounter model (REM) and camera trap distance sampling (CTDS). Both models need to account for variation in animal behavior that depends, for example, on the species and sex of the animals along with temporally varying environmental factors. We examined whether the density estimates of REM and CTDS can be improved for Europe’s most numerous deer species, by adjusting the behavior-related model parameters per species and accounting for differences in movement speeds between sexes, seasons, and years. Our results showed that bias through inadequate consideration of animal behavior was exceeded by the uncertainty of the density estimates, which was mainly influenced by variation in the number of independent observations between camera trap locations. The neglection of seasonal and annual differences in movement speed estimates for REM overestimated densities of red deer in autumn and spring by ca. 14%. This GPS telemetry-derived parameter was found to be most problematic for roe deer females in summer and spring when movement behavior was characterized by small-scale displacements relative to the intervals of the GPS fixes. In CTDS, density estimates of red deer improved foremost through the consideration of behavioral reactions to the camera traps (avoiding bias of max. 19%), while species-specific delays between photos had a larger effect for roe deer. In general, the applicability of both REM and CTDS would profit profoundly from improvements in their precision along with the reduction in bias achieved by exploiting the available information on animal behavior in the camera trap data.
What the paper shows and why it matters
(AI-generated)
Camera traps can estimate the density of animals that cannot be told apart individually, from the rate at which animals trigger the cameras. The random encounter model (REM; Rowcliffe et al. 2008) uses an average movement speed, often derived from telemetry data. Camera trap distance sampling (CTDS; Howe et al. 2017) instead counts animals at fixed “snapshot” moments and derives movement information from the camera data. Both rest on parameters that describe behaviour, and these vary: speed differs between sexes, seasons and years, animals may react to the cameras, and photo delays differ between species. Single sources of such bias had been discussed, but the paper notes that a systematic analysis was lacking. It asks how large they are, and how they compare with the imprecision of the estimates.
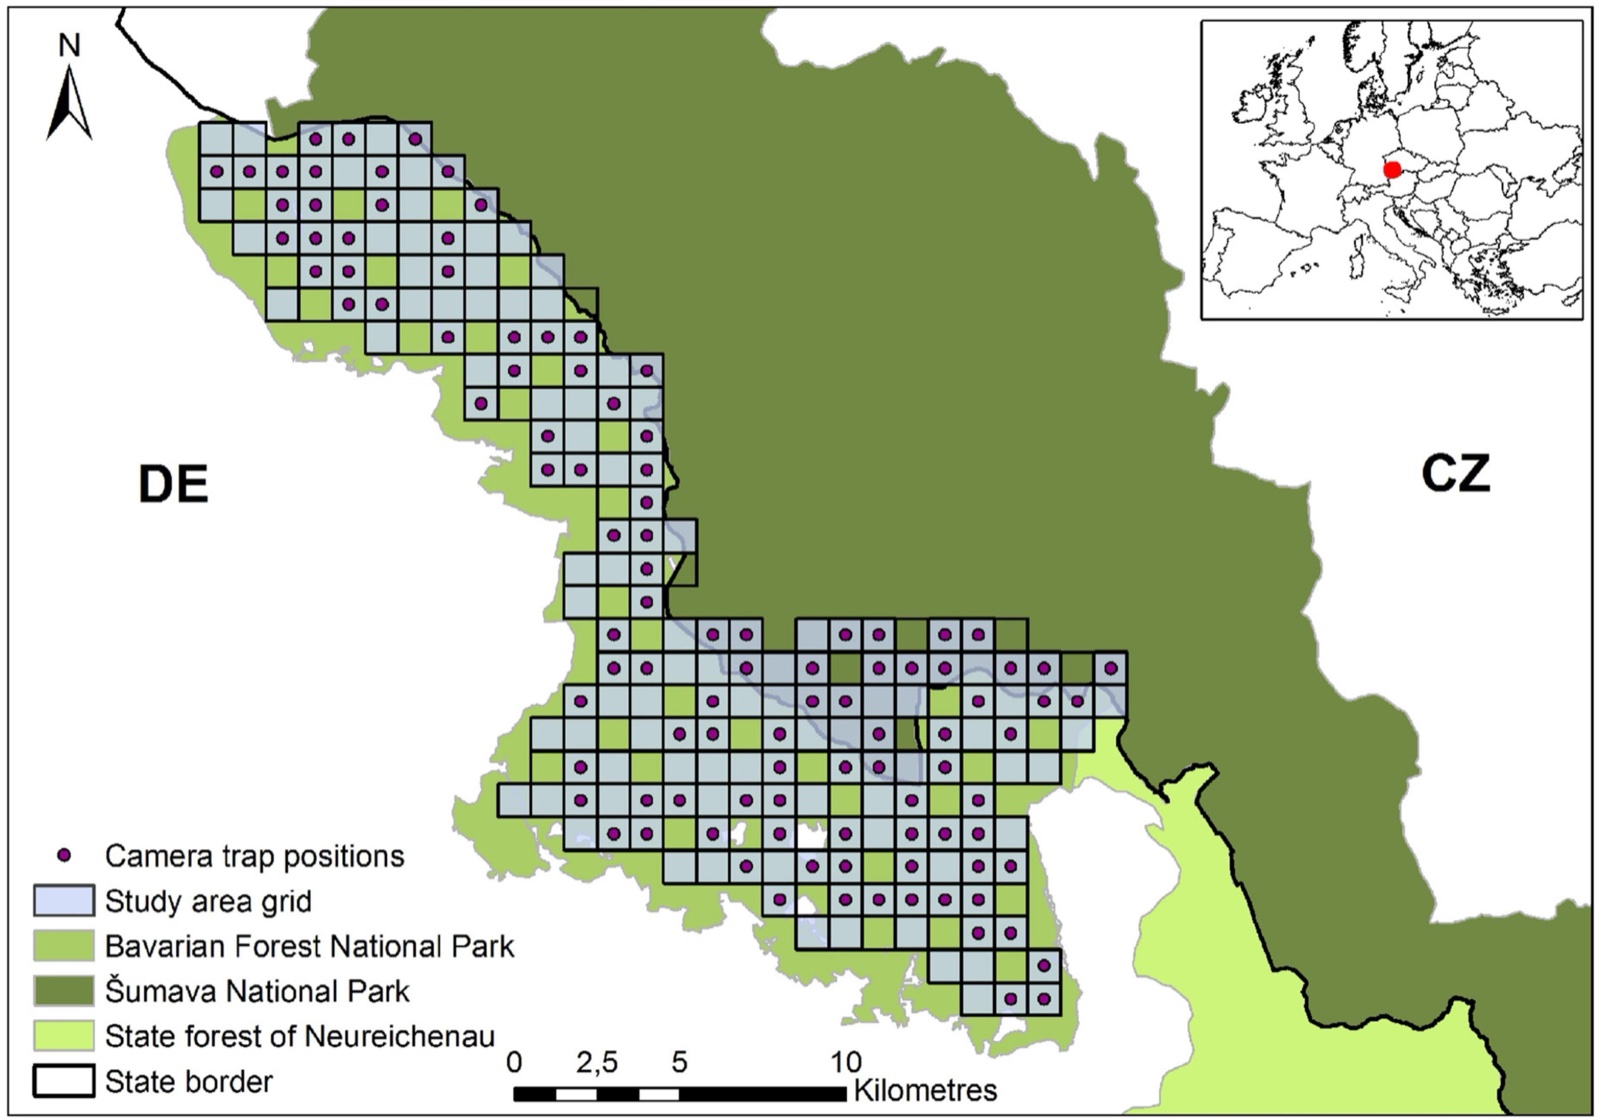
The paper finds that behaviour-related bias in camera-trap density estimates can be sizeable (up to 19% here) but is outweighed by imprecision, which stems mainly from differences in trapping rates between camera locations. The test case is a year of data from 108 cameras in the Bavarian Forest and Šumava national parks, on red and roe deer, with GPS telemetry. Ignoring seasonal differences in movement speed overestimated red deer density in REM by ca. 14% in autumn and spring. In CTDS, ignoring red deer’s reactions to the cameras caused biases of up to 19%, and ignoring species-specific photo delays overestimated roe deer density by 14%. None of these biases, alone or combined, was significant: the bootstrap confidence interval of each shift from the reference estimate included zero. In REM, differences in trapping rates between locations explained at least 65% of the variance in the estimates, except for both species in spring; in CTDS, other parameters sometimes mattered more.
The paper reads these results as an argument for using behavioural information already in the camera data: it advises caution with GPS-derived speeds in REM and recommends species-specific photo delays in CTDS. It argues that better precision is a prerequisite for detecting small changes in density, and suggests more camera locations, accounting for habitat selection in the models and automated image processing as ways to get there. If behaviour is considered properly and precision improves, the paper argues, both methods could become reliable and feasible tools for regular monitoring of common ungulates.
References
- Rowcliffe et al. (2008). Estimating animal density using camera traps without the need for individual recognition. Journal of Applied Ecology 45, 1228–1236. doi:10.1111/j.1365-2664.2008.01473.x
- Howe et al. (2017). Distance sampling with camera traps. Methods in Ecology and Evolution 8, 1558–1565. doi:10.1111/2041-210x.12790